Proteins are always moving. They wiggle. They jiggle. They interact with their surroundings. That movement drives their function.
Yet the motion stays mostly invisible. We cannot understand protein function, engineer it, or correct it until we can see the motion and predict it. https://t.co/jLsPrJmvR7
New in BANDICOOT: color each altloc a distinct hue, so you see heterogeneity while you build. Each added alternate conformation is auto hue-shifted from the last; remove them all and the residue returns to bulk color. Configurable and open source! https://t.co/WH2TxZB19P #compbio
In a test case, swapping Phenix's flat bulk-solvent mask for an MD-derived map lowered cross-validated R-free from 0.147 to 0.109 in one 0.96 Å. Code here: https://t.co/Gex7Baz1lk
Bulk solvent fills ~half a protein crystal. Modeling this is required for a good fit to experimental data. How best to model this remains an open question. New from diffUSE: a Phenix patch to supply your own solvent map (MD, 3D-RISM, EDEN, neural nets). https://t.co/N0sRw0q9rC
Our review on AI for protein engineering is out now, about this too-fast-moving field full of hype and overclaim, yet one that is having a real impact on the world and can be described in a coherent manner without histrionics
https://t.co/woOWuyTV5R
Our new ICLR paper on leveraging “soft decomposability” of design spaces (eg protein sequence) wrt a target property (eg enzymatic activity) in order to more efficiently search through the design space. Active site vs. scaffold, for eg. @jamesbowden_ joint with @svlevine
Our new paper on leveraging ML to characterize the fitness landscape of two proteins binding through evolution, wrt geometry, epistasis, etc. The super hard work of Hanlun Jiang, Stephan Allenspach and @jamesbowden_ on our end. https://t.co/qtrURlRYyM
New, full length ProteinGuide manuscript, now spanning interpolative, extrapolative and multi-property (extending Pareto optimality) settings; comparisons to fine-tuning; and beating 7 rounds of directed evolution with just one round of ProteinGuide.
https://t.co/wIexIhNow2
Delighted to share our publication in @NatureComms on the computational design of generalist carbene transferases with tailored, stereodivergent selectivity! Great collab with Sagar Khare! Kudos to Zhuofan, Mary, and Xinkun and all other coauthors!
https://t.co/YAtfzLI0np
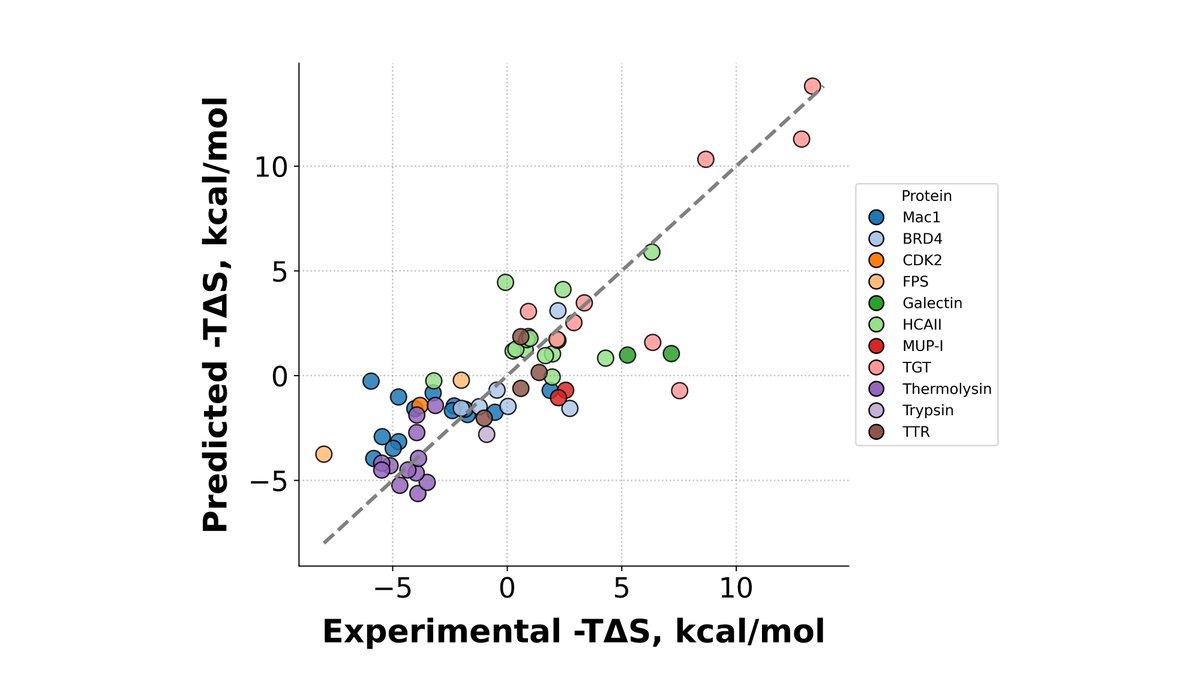
New Preprint!! We show that binding entropy can be quantitatively predicted from crystallographic ensemble models, accounting for both protein conformational entropy and solvent entropy! https://t.co/h9L4glyBYr
https://t.co/SSytLwl6i1... most proteins are multi domain but our understanding of how architectures evolve is limited - we mapped 40K chitinases and show a stepwise grammar of domain gain/loss and localisation changes that predicts ecological strategy and physiological function
Protein design mostly targets single domains; but bio builds function by recombining domains into larger multi domain proteins. Understanding the evolutionary rules of domain assembly will be important if we want to design the level of functionality seen in many native proteins
‘Protein evolution as a complex system’ – A new Comment discusses protein evolution in terms of complex systems theory and machine learning approaches to model the dynamics of protein evolution
https://t.co/L62p40MOQh
Really proud of this work by Jae Kennemur and Yueming Long. #Enzymes rock, with a little help from #directedevolution to do #chemistry not known in nature (and not easily done by humans).